When Colon Cells Begin to Use Fuel Differently
Healthy, mature colonocytes normally obtain much of their energy through mitochondrial oxidation. Microbial butyrate is converted into acetyl-CoA and used in pathways that consume oxygen and efficiently generate cellular energy.
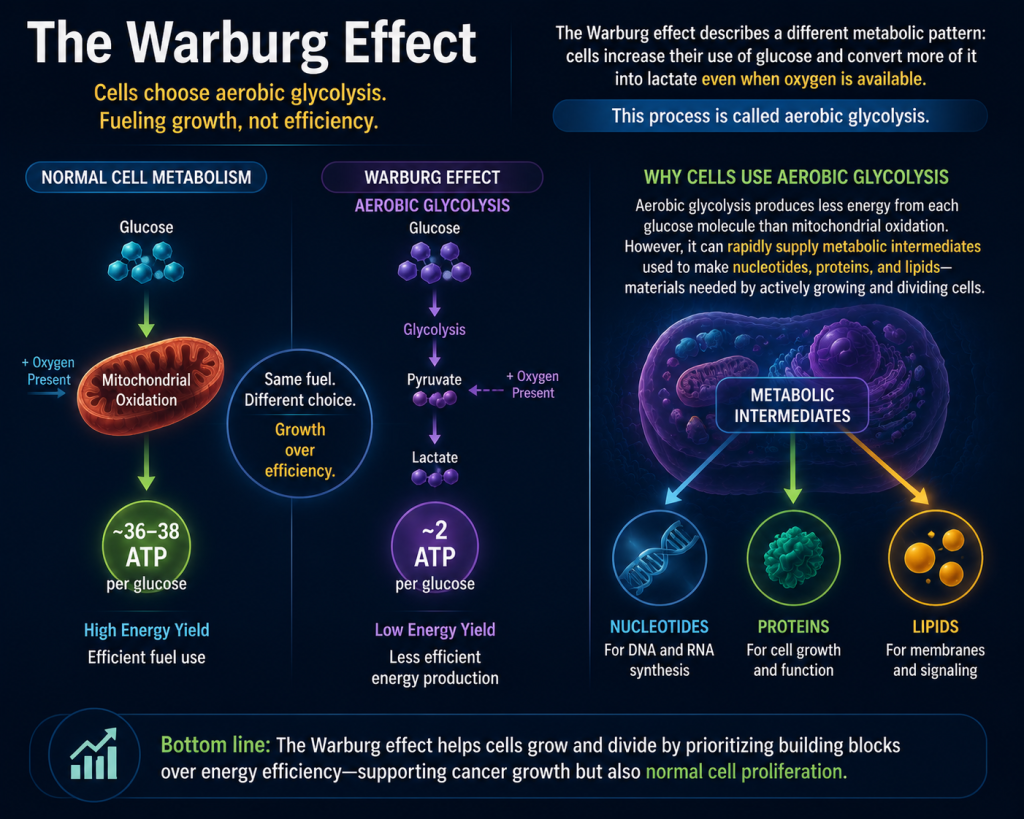
The Warburg effect describes a different metabolic pattern: cells increase their use of glucose and convert more of it into lactate even when oxygen is available. This process is called aerobic glycolysis.
Aerobic glycolysis produces less energy from each glucose molecule than mitochondrial oxidation. However, it can rapidly supply metabolic intermediates used to make nucleotides, proteins, and lipids—materials needed by actively growing and dividing cells.
A Warburg-like shift does not mean that mitochondria have simply stopped working. Glycolytic and mitochondrial metabolism can coexist, and their relative contributions vary among cells and over time.
What May Predispose the Colonocyte – Warburg Conversion?
The development of the Warburg effect in colonocytes is likely influenced by multiple interacting biological processes rather than a single event. A diet low in dietary fiber and resistant starch provides less fermentable substrate to the gut microbiome, reducing the growth and activity of beneficial butyrate-producing bacteria. As microbial diversity declines, butyrate production falls, depriving colonocytes of their preferred mitochondrial fuel and reducing oxidative metabolism.
Loss of efficient butyrate oxidation may increase reliance on glucose metabolism and aerobic glycolysis, establishing the metabolic pattern known as the Warburg effect. This metabolic shift is accompanied by changes in gene expression, mitochondrial function, and cellular signaling that may promote abnormal proliferation, impaired differentiation, and reduced cellular resilience.
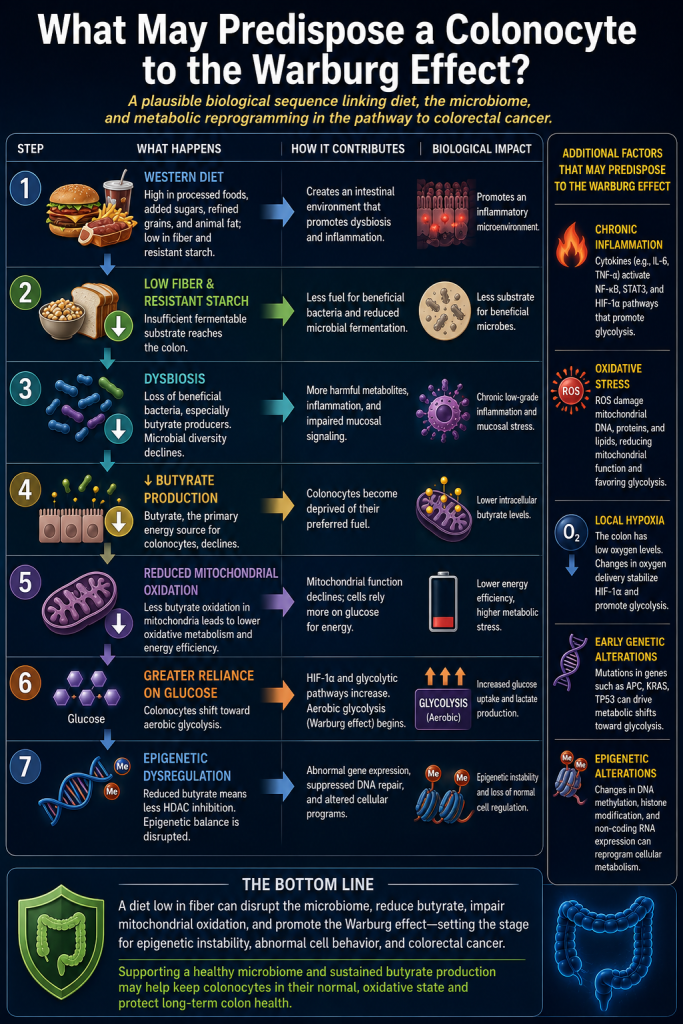
Additional biological factors may reinforce this process. Chronic inflammation activates signaling pathways such as NF-κB, STAT3, and HIF-1α that favor glycolysis, while oxidative stress damages mitochondrial proteins, lipids, and DNA, further reducing oxidative metabolism. The naturally low-oxygen environment of the colon may stabilize HIF-1α, encouraging glycolytic metabolism, and early genetic or epigenetic alterations may further shift cellular energy production toward aerobic glycolysis.
Although the precise sequence of these events has not yet been established, current evidence supports the concept that diet, the gut microbiome, microbial metabolites, mitochondrial function, inflammation, and epigenetic regulation interact to influence colonocyte metabolism. Within the EpiNutrition™ framework, maintaining a healthy microbiome through adequate dietary fiber and resistant starch may help preserve butyrate production, support normal mitochondrial oxidation, and reduce the likelihood of metabolic reprogramming that precedes colorectal neoplasia.
Evidence of an Early Metabolic Change in Normal-Appearing Colon Tissue
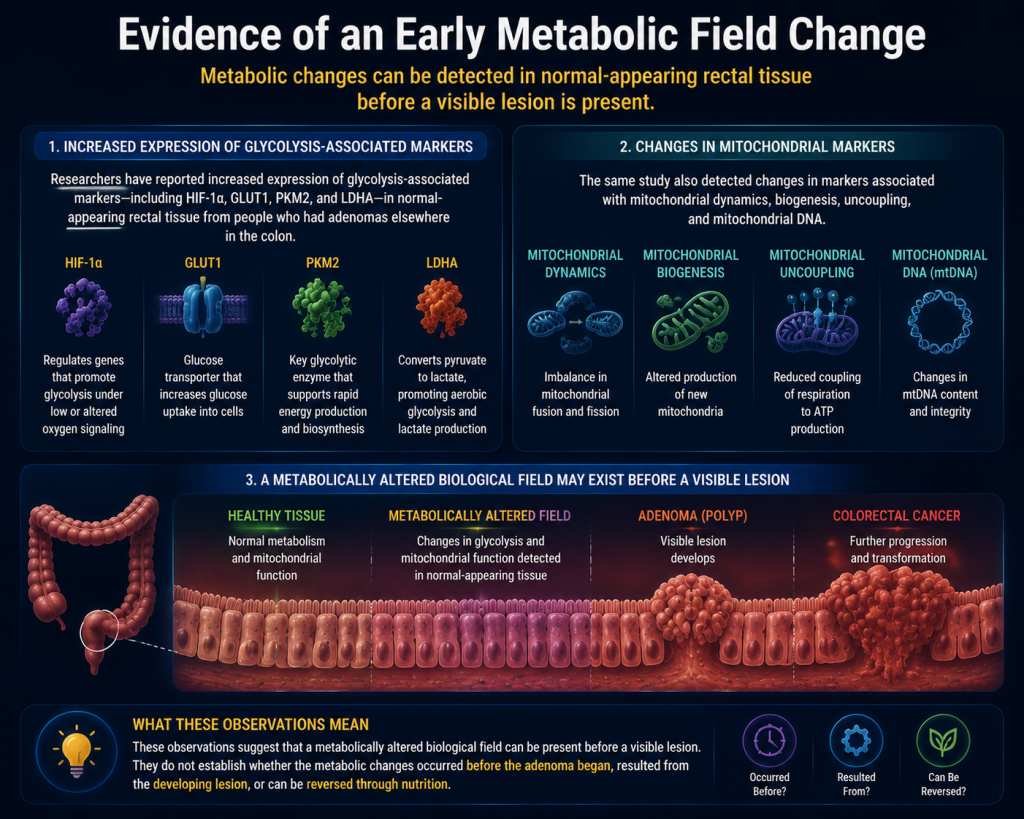
Researchers have reported increased expression of glycolysis-associated markers—including HIF-1α, GLUT1, PKM2, and LDHA—in normal-appearing rectal tissue from people who had adenomas elsewhere in the colon.
The same study also detected changes in markers associated with mitochondrial dynamics, biogenesis, uncoupling, and mitochondrial DNA.
These observations suggest that a metabolically altered biological field can be present before a visible lesion. They do not establish whether the metabolic changes occurred before the adenoma began, resulted from the developing lesion, or can be reversed through nutrition.
Why the Warburg Effect Matters
Healthy colonocytes normally rely on butyrate, produced by the gut microbiome, as their primary energy source. Within the mitochondria, butyrate is efficiently oxidized to generate ATP, providing the energy needed to maintain the intestinal barrier, support continuous cellular renewal, regulate inflammation, and preserve normal gene expression.
In contrast, colonocytes that undergo metabolic reprogramming increasingly depend on glucose metabolism through aerobic glycolysis, a process known as the Warburg effect. Although glycolysis allows cells to generate metabolic building blocks rapidly, it produces much less ATP than mitochondrial oxidation and reduces the cell’s ability to utilize butyrate as its primary fuel.
As mitochondrial oxidation declines, butyrate is no longer completely metabolized for energy and can accumulate within the cell. At the same time, increased glycolysis produces lactate and contributes to a more acidic cellular environment. These metabolic changes are associated with increased oxidative stress, impaired DNA repair, altered epigenetic regulation, abnormal cell proliferation, reduced cellular differentiation, and weakening of the intestinal barrier.
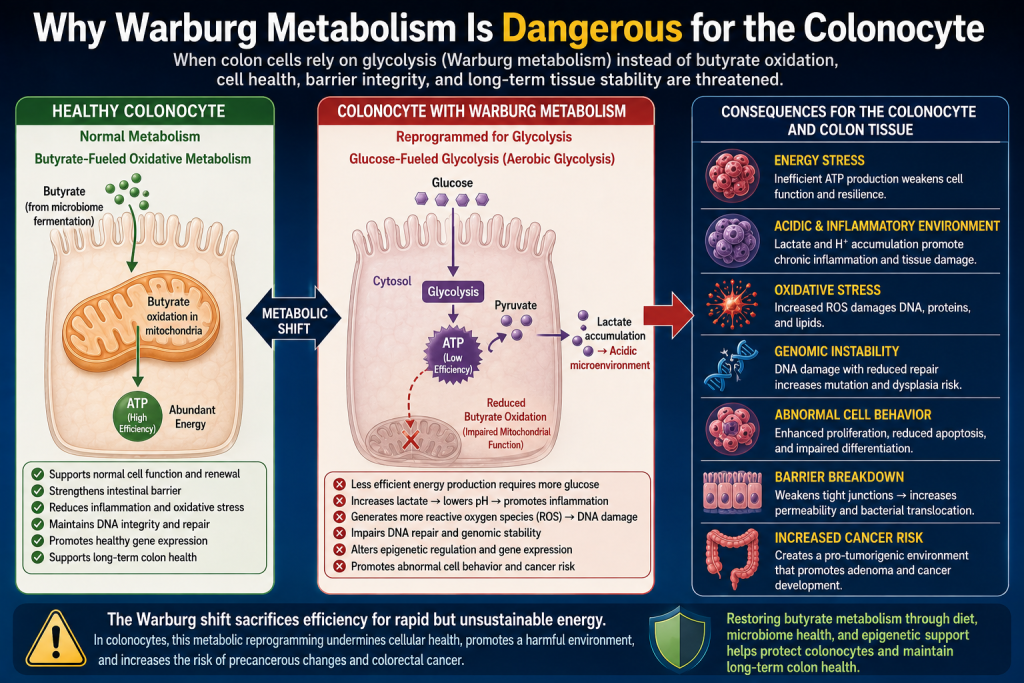
Together, these changes create a biological environment that is more susceptible to chronic inflammation, genomic instability, and the development of colorectal neoplasia. Rather than simply representing a change in energy production, the Warburg effect fundamentally alters the way colonocytes respond to microbial metabolites and regulate gene expression.
These observations help explain why maintaining healthy microbial production of butyrate—and preserving the colonocyte’s ability to oxidize it—may be an important component of long-term colon health. Within the EpiNutrition™ framework, nutrition supports a healthy microbiome, the microbiome produces beneficial metabolites, and those metabolites help maintain normal colonocyte metabolism and healthy gene expression long before visible disease develops.
Can Butyrate Reverse the Warburg Effect?
A growing body of experimental research suggests that butyrate may help counteract key features of the Warburg effect in colorectal cancer cells. Unlike healthy colonocytes, which readily oxidize butyrate within their mitochondria, many colorectal cancer cells rely heavily on aerobic glycolysis. In these metabolically reprogrammed cells, reduced mitochondrial oxidation allows butyrate to accumulate rather than being completely used as fuel.
This intracellular accumulation enables butyrate to function as a natural histone deacetylase (HDAC) inhibitor, altering the expression of numerous genes involved in cellular metabolism, differentiation, cell-cycle regulation, and programmed cell death. Experimental studies have shown that butyrate can reduce glycolytic activity, promote mitochondrial oxidative metabolism, increase cellular differentiation, slow proliferation, and stimulate apoptosis in colorectal cancer cell lines and animal models. Together, these changes oppose many of the biological characteristics associated with the Warburg phenotype.
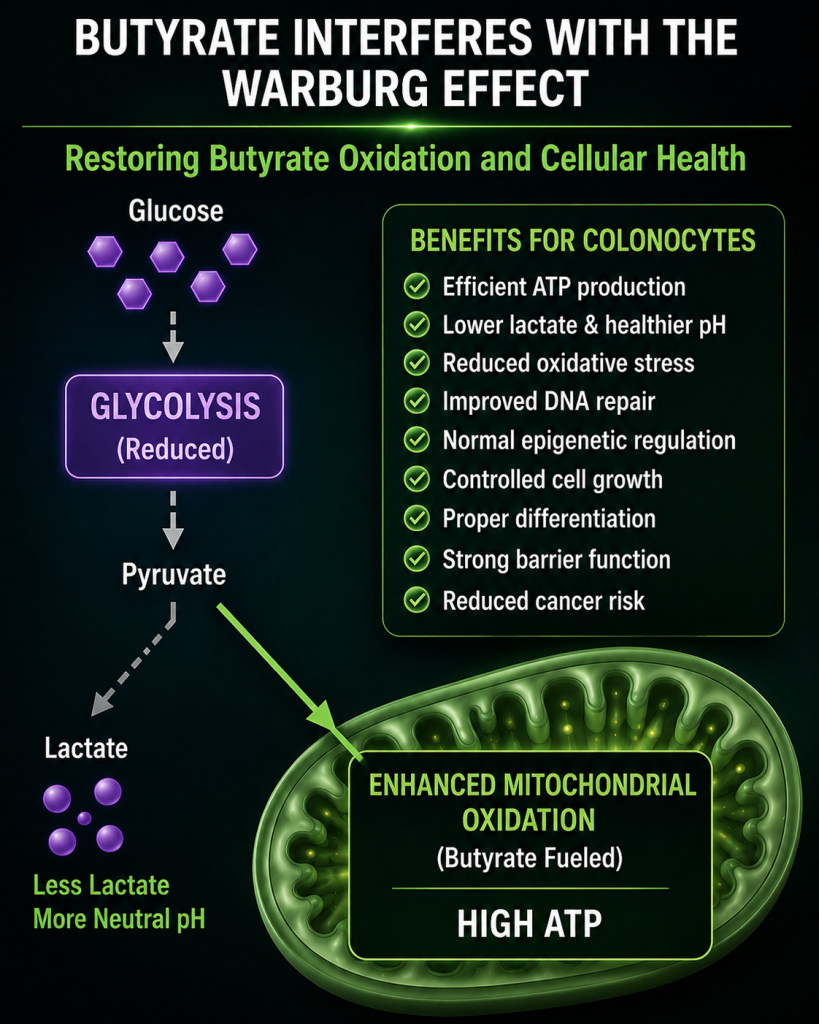
Importantly, these findings have been demonstrated primarily in cell culture and experimental animal models. Although they provide compelling mechanistic evidence that microbial metabolites can influence cancer cell metabolism, they do not establish that dietary interventions or increased butyrate production can reverse the Warburg effect in humans with established colorectal cancer. Additional clinical studies are needed to determine whether these experimental observations translate into meaningful therapeutic benefits.
Within the EpiNutrition™ framework, these studies illustrate an important biological principle: microbial metabolites are not simply nutrients—they are signaling molecules capable of influencing the metabolic state of colonocytes. By supporting a healthy microbiome and sustained butyrate production, nutrition may help maintain normal cellular metabolism and healthy gene expression long before visible disease develops.
References
- Vander Heiden MG, Cantley LC, Thompson CB. Understanding the Warburg effect: the metabolic requirements of cell proliferation. Science. 2009;324(5930):1029–1033. doi: 10.1126/science.1160809. PMID: 19460998; PMCID: PMC2849637.
- Donohoe DR, Collins LB, Wali A, Bigler R, Sun W, Bultman SJ. The Warburg effect dictates the mechanism of butyrate-mediated histone acetylation and cell proliferation. Molecular Cell. 2012;48(4):612–626. doi: 10.1016/j.molcel.2012.08.033. PMID: 23063526; PMCID: PMC3513569.
- Dela Cruz M, Ledbetter S, Chowdhury S, Tiwari AK, Momi N, Wali RK, et al. Metabolic reprogramming of the premalignant colonic mucosa is an early event in carcinogenesis. Oncotarget. 2017;8(13):20543–20557. doi: 10.18632/oncotarget.16129. PMID: 28423551; PMCID: PMC5400525.